Field of Science

What songbirds can teach us about language: Does syntactic complexity require selection?

[since I had to write this up elsewhere for a class, might as well double post this here anyway]

Here's another story of how alleviated selective pressures can enable increased complexity, without said increase in complexity needing to be driven by positive selection; the paper later relates this to its implications for language evolution:

Ritchie & Kirby 2005 Evol Ling Comm Selection, domestication, and the emergence of learned communication systems
(Also see Ritchie & Kirby 2007
Emergence of Communication and Language)

In a prior study, the Bengalese finch was found to have a more complex song syntax than its wild ancestor (the white-backed munia); furthermore, while the finches could learn the songs of munia, the latter could not effectively learn the complex songs of the finches, suggesting that a part of the capability was physiological. The author of that prior study, Okanoya (2002), argued that the song complexity in the Bengalese finch was driven through sex selection, as the more basic pressures (food and predation) were relieved by domestication, enabling sex selection to finally drive up the complexity; furthermore, this would have been an honest signal of the male’s fitness, as a fitter bird could produce a more complicated song.

A competing hypothesis by Deacon agrees that song complexity is kept low in the wild munia through selective pressure, but claims that the lifting of basic selective pressures after domestication enabled the songs to get more complex through other means, namely drift. Thus, processes that previously paled in comparison with the selective pressures against excess song complexity became prominent, such as the effect of songs heard at an early age and mnemonic biases; that is, songs with a more regularised syntax may be easier to recall. Deacon further extends this concept to the evolution of human language; he calls the concept “selective masking”. In short, complexity may arise in the finches’ songs without being driven by direct selective pressure.

Ritchie and Kirby set out to test the competing hypotheses through computational modeling; long story short, a bunch of learning filters are set up amid evolutionary models, and the simulation is run trough three phases: 1) Population is filtered to have a particular song type; variation is reduced (modeling the case among wild munia. 2) The population, having learned (and become “attached” to) a particular kind of song, is now bombarded with a bunch of random songs, and demonstrates resistance to be affected much by it: the simulated birds still learn the ‘correct’ song over incorrect ones. 3) Selective pressure is alleviated altogether by simply ceasing to calculate the fitness values. This simulates domestication. Population was once again bombarded with random songs.

Complexity was initially defined by Okanoya as the number of unique song notes divided by the number of unique note-to-note transitions (aka ‘Song Linearity’); Okanoya found this ratio to be lower in the Bengalese finches than the wild munia, meaning their songs were more complex (less ‘linear’). Ritchie & Kirby’s simulation also yielded similar results; though they argue that a completely random song would have the maximum complexity by such measures. Additionally, they also used Grammar Encoding Length, or the number of bits required to describe a [in this case, Probabilistic] Finite State Machine, which was used to model song learning. [Now the structural linguistics and information theory loses me completely...]. Turns out, in phase 3, the grammar encoding length did increase and the linearity did go down, supporting the increase in song complexity after domestication.

Most importantly, their simulation showed that song complexity can increase in the absense of direct selective pressure, as selection was eliminated altogether in phase 3. This suggests that [once again,] one need not necessarily evoke often-absurdly-complex selection stories (like sex selection and ‘honest signals’) to explain the song complexification in Bengalese finches. Furthermore, these results can be extrapolated further to linguistic evolution, suggesting that perhaps not all of syntax complexification requires selective pressures behind it. In fact, the eliviation of such pressures can allow more complex syntax to arise. As a sidenote, it has been observed that the rise of writing resulted in higher complexity of clause embedding, and this complexity also rose gradually, not immediately after writing systems first appeared (Karlsson in Sampson et al. 2009 Language Complexity as an Evolving Variable). This can also be seen as a case of the lifting (aka ‘masking’) of a selective constraint resulting in allevated complexity, in this case probably not particularly adaptive either. One can convey complex ideas just as well, and in some cases better, without the [ab]use of intricate clausal embedding…

Ritchie and Kirby conclude with an idea that perhaps one mustn’t look for selective advantages of elaborate syntax found in human language, but instead investigate what may have prevented syntactic elaboration from arising in the past – what selective pressure may have been alleviated, and what may have caused them?

Ritchie GRS, & Kirby S (2007). A Possible Role for Selective Masking
in the Evolution of Complex, Learned
Communication Systems Emergence of Communication and Language, 387-401 DOI: 10.1007/978-1-84628-779-4_20

(Ritchie + Kirby 2005 turns out to be a draft for the 2007 paper, and I'm far too sleepy to reference that properly as it's too complicated...)

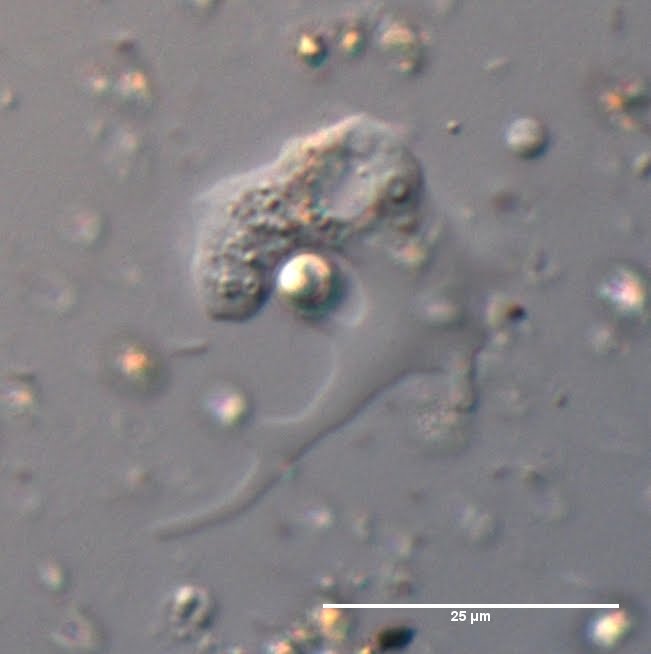
Mystery Micrograph #20

Originally posted at 00:31 31 Mar 2010
You guys are too good at this...next!
(Oh, and I am working on writing up the past ones... just so you know -- they're coming, eventually...)

Scalebar = 25um; to be referenced later

Edit [20 Apr 2010]: Figured another image may help:

Scalebar = 500um; to be referenced later

Poor thing's been feeling rather neglected lately. Never underestimate the dangers of a microorganism gone mad from abandonment...

Edit [24.04.10]: Another glimpse.
Scalebar = 10um; to be referenced later

I'd like you to pay particular attention to the surface structure... /hint

Sunday Protist -- Gymnodinium catenatum: Like beads on a string

I'm going to be genuinely lazy today. Seriously cannot go off on a 3h literature journey looking at random protists with an invert zool final happening so very soon (Monday). Even though the instructor is actually a protistologist. Maybe his final will let me ramble about choanoflagellates somewhere...

Today we have some random dinoflagellates; well, not as much random as rather 'typical' for the group, although with an interesting tendency to form long chains, which is not so typical. Meet Gymnodinium catenatum, a concatenated naked dinoflagellate:
Gymnodinium is photosynthetic, and has an unfortunate side effect of producing chemicals humans and other animals find toxic. Despite the occasional public mania on the topic, not all dinoflagellates do this, and those who do didn't really mean to, and would perhaps even write a letter of apology were they capable of and interested in such a thing. Also, algal blooms have been happening for millions of years and are not a 'new' thing by any means. Just that nobody 'noticed' until we came alone and started writing about it. That said, harmful algal blooms are an important research topic, but probably the efforts should be directed to finding antidotes and other medical solutions to the problem, and educating the public instead of causing panic, rather than naive attempts at eradicating blooms altogether. But that's just my entirely non-expert opinion. Yeah, I personally don't find that topic particularly fascinating, and am kind of annoyed by the majority of dinoflagellate papers seeming to be about their toxicity and blooms instead of their biology and evolutionary history. Meh.

Seriously, look how cute dinos are! There's quite a few extreme oddities in the group as well, and I'll leave them for later. Previously, I've touched on the morphologically awesome dinophysis, ferocious palium-feeding Protoperidinium that eats things bigger than itself, and Ceratium which grows plastid-filled 'fingers' during the day and retracts the plastids and fingers during the night. I still haven't touched on the really weird stuff though! It shall happen eventually...

Ok, back to dreading finals and life in general. Just two weeks. I can do this...I think.

Moss Microforay Part 1: Assorted critters

Posting and attempting to identify own micrographs is a quick and easy way to fill up blog posts when one is short on time. Aside from all the time spent at the scope and processing the images (ImageJ, baby!) of course. At least there's no expiry date on these, unlike hot new topics which need to be blogged within an hour else the entire blogosphere will scoop you, somehow...

Moss was sampled on a coastal mountain on the San Francisco peninsula. As the sampler is a labrat and therefore not particularly sample-savvy, said specimen was abandoned for three weeks only to be rehydrated a couple days prior to imaging. Thus, there is a high probability that much of the really cool stuff died off before I got around to it. Conversely, some of that cool stuff may be damn good at encysting, and is now perhaps freshly-excysted.

Saving the Euglyphids for the next installment. Mwahaha. Let's go over an assortment of random non-Euglyphid organisms first. It would be nice to get some help with ID from the experts lurking here *wink*

Ok, first off -- flagellates. That is, glimpses of the few flagellates that weren't moving so ridiculously fast they were but a blur on the picture. There seemed to be a lot of bicoesid-like loricate things (or vaguely look like them anyway):

That cell may have been damaged somehow, or is it actually being amoeboid-ish? Can bicoesids do that? My understanding is they tend to be rather rigid, but I'm not aware of any other loricate flagellate besides Dinobryon and choanoflagellates. This thing is definitely neither of those.

This specimen appeared attached along the length of the flagellum at the top of the picture.


This one looks more like a bicoesid. As do the next three:


This one too, probably, though the lorica can't be seen. There are aloricate bicoesids as well.

Bicoesids are actually borderline suitable for microphotography with a slow camera due to their habit of attaching to things. Seriously, sessile organisms are really nice that way...

More potentially cool flagellates that were moving around too much to get a decent shot:


This was a sequence following a strange amoeboflagellate-looking thing(s) -- any idea what this may be? A cercomonad of sorts?

Same cell(s) in all of the images. Was shot in a short timeframe (maybe a minute or two), so highly doubtful that cell divison could've occured within that time. Or maybe not?

Amoebozoan time! May ever try ID'ing some...before doing that, I feel compelled to draw your attention to Smirnov & Goodkov 1999 Protistology, a wonderful overview of and reference for amoeboid morphotype diversity -- amoebae do have shape! Another good source for ID'ing amoebae is Smirnov & Brown 2004 Protistology, and an associated site (though sadly not maintained since 2003ish =( ); I will be relying on those to see how far I can go:

This one seems to be flabellate with adhesive uroidal filaments; may be Flabellula (something off about that), Stachyamoeba (perhaps? esp. this picture); Rosculus seems to lack prominent uroidal filaments as well as seemingly a Heterolobosean from what I've gathered. Could also be of the fan-shaped morphotype but those don't seem to leave trailing adhesive filaments that much. I'll go with Stachyamoeba for now, hopefully no one finds that offensive...

Ok, the next one is probably polytactic or dactylopodial by morphotype.

Candidates: Amoeba (too small), Chaos (doesn't seem multinucleate and huge), Deuteramoeba, Thecochaos (not wrinkly enough), Polychaos (something meh about that too). As for dactylopodial candidates, Paramoeba is looking better, as is Korotnevella. As the former is much more commonly mentioned, I'll go with Paramoeba for this one.

By the way, the prominent round thing in the middle is most likely the contractile vacuole; note how it obvious changes size during optical sectioning, especially in the first specimen. Also, amoebae aren't always amoeboid -- many species take upon 'floating forms' which tend to look like spiky balls. Some amoebae are apparently quite at ease with being planktonic too, like this vicious rotifer-munching Difflugia mentioned earlier.

Amoebae can actually move pretty quickly -- this one is fuzzy due to motion blur.

Morphotype: Lens-like (Smirnov & Brown 2004); candidate: Cochliopodium (and here). Really does look like Cochliopodium; perhaps I got at least one right!

A few more fun amoebae:

In the last one, note how the clear pseudopodia emphasising the contrast between ecto- and endoplasm -- the latter being fairly gelatinous and containing the 'stuff' of the cell; the former, full of actin, responsible for cell motility.

Arcellid amoeba: (proteinaceous test -- note texture)


Odds and ends: First off, ???:


What I think might be a developing nematode egg case (elsewhere there were very similar things with nematodes inside):


Some fungal thing? (germinating spore?)


And last but not least for today, a bacterial filament:


Ok, back to cramming...stay away, internet! Must know everything there is to know about invert biol by Monday...aaaah~! Also, apparently metazoan phylogeny is in about as much of a mess as the the Tree of Eukaryotes. Kind of creepy...

In defense of constructive neutral evolution - Part II

ResearchBlogging.orgContinued from Part I here

Part I
- Adaptationism vs. Neutralism
- "Population genetics ignores reality!"
- Existence of neutrality and near-neutrality
Part II
-Neutral evolution is relevant
-Evolution lacks foresight; it can neither anticipate nor respond
-Clarifying some terminology: two types of function, positive vs. negative selection
-Rise of complexity through non-adaptive means
-An example of constructive neutral evolution at work: loss of group I intron self-splicing
Part III
-Further examples of constructive neutral evolution
-Discussion of what sparked this argument: Evolution of ciliate nuclear dimorphism

Neutral evolution is relevant

Again, apologies for stating the obvious, but apparently even some prominent evolutionary biologists popularisers of evolutionary biology fail to grasp this simple concept. I've masticated this point to a fine mush by now, but selection and neutral processes act in tandem. Mutational bias and drift matter. So often in the literature you find people arguing over whether something is an adaptation or a spandrel. This gets even more absurd when the structure in question is as massive as the human language capacity. For example, in the landmark Pinker & Bloom 1990 paper signalling the revival of evolutionary linguistics, you find awful sentences like:
"The key point that blunts the Gould and Lewontin critique of adaptationism is that natural selection is the only scientific explanation of adaptive complexity." [p.6; emphasis mine]
First off, it's kind of cute that a couple psychologists seem to think they can so easily outright dismiss a point made by evolutionary biologists. I mean, seriously, I find it adorable. On that note, I'm now gonna write a book chapter debunking generative linguistics, because, well, my buddy says they're wrong. I wonder how much Pinker's evolutionary views have been shaped by Dawkins et al. Their camp is rather influential outside evolutionary biology, and while many claim that panadaptationism is a strawman -- and even in biology that point is debatable -- outside evolutionary biology, panadaptationism is alive and well. Part of the reason is that adaptationist stories are written in popular books, while pluralistic approaches largely remain hidden in the likes of Molecular Biology & Evolution, Biology Direct and Journal of Molecular Evolution. Researchers working in applied evolutionary fields have likely never heard of them.

Back to Pinker & Bloom, first off it's quite a tautology to claim that adaptive complexity evolves through adaptation. Well, yes, you JUST labelled it adaptive. In the immortal words of 4chan, long cat is loooooong. Casting that aside, they've falled for a false dichotomy. You would think someone as smart as Steven Pinker and Paul Bloom wouldn't fall for it. But they did. Why does it have to be one or the other? Why adaptation or spandrel? Especially when we speak of highly complex systems -- is it not in the definition of complexity that they consist of multiple components? How likely is it that all of them are adaptive or neutral or maladaptive? Is it even remotely productive to reduce a system so drastically as to label it simply as an adaptation? What does that even mean, besides stating the obvious? 'Adaptation' has got to be one of the more utterly useless terms in evolution biology, at least the way it's abused today.

Letting Pinker & Bloom speak further:
"Adaptive complexity" describes any system composed of many interacting parts where the details of the parts' structure and arrangement suggest design to fulfill some function. The vertebrate eye is the classic example. The eye has a transparent refracting outer cover, a variable-focus lens, a light-sensitive layer of neural tissue lying at the focal plane of the lens, a diaphragm whose diameter changes with illumination level, muscles that move it in precise conjunction and convergence with those of the other eye, and elaborate neural circuits that respond to patterns defining edges, colors, motion, and stereoscopic disparity. It is impossible to make sense of the structure of the eye without noting that it appears as if it was designed for the purpose of seeing -- if for no other reason that the man-made tool for image formation, the camera, displays an uncanny resemblance to the eye. Before Darwin, theologians, notably William Paley, pointed to its exquisite design as evidence for the existence of a divine designer. Darwin showed how such "organs of extreme perfection and complication" could arise from the purely physical process of natural selection." [p.6 cont'd]
Holy fucking crap, argument from design, for selectionism! Impressive. Yes, you guys just totally pwned Gould with the vertebrate eye. He was unaware of its very existence. Eyes don't preserve well in the fossil record, you see? Eyes look designed, therefore selection. Great. I'll let them finish...
"The essential point is that no physical process other than natural selection can explain the evolution of an organ like the eye." [p.6]
AFAIK, Gould never denied selection!!! He was a brilliant biologist who thoroughly understood evolution, unlike some recent drama queens. What Gould argues is that a) not everything is an adaptation and b) adaptation is neither the sole nor the most important 'force' in evolution (nor is it actually a 'force' of any sort...). Furthermore, while I am unaware of Gould's opinions about The Eye, and am currently too lazy to research the topic, to me it seems highly implausible that the vertebrate eye evolved solely through selection. In fact, considering that selection is a purifying, not driving, 'force' -- that is, selection simply removes the not sufficiently fit -- it is curious to see where Pinker & Bloom think the 'material' for the selective evolution of the eyes comes from. Surely they're not insane enough to believe that the thing evolved entirely through point mutations each making the eye progressively slightly better and better and suddenly, veeeery gradually, ta-da: The Eye!

On that note, I wonder if there's a strong link between selectionism and gradualism. In a sense, one does kind of have to believe the above point-by-point scenario to explain how anything arises purely by selection. To anyone with the slightest inkling of how genes and genomes work, such a view is obviously absurd. Although considering how Dawkins has already enlightened us that molecular biologists may or may not be -reputable- biologists...

I'm still amused by how remarkably cute it is of Pinker & Bloom to know so much about the details of evolution that they can make bold statements like the last sentence cited above. That's one strong statement!

tl;dr Some rather reputable and smart people still fall for the false dichotomy where something is either purely adaptive or purely 'random'. Selection is not the sole source of order (Lynch 2007 PNAS; you might as well head over and read that paper by now)

So if selection is not the only source of order, what else could be? How can neutral forces (coupled with negative selection) result in an increased complexity? Ah, nearly time for constructive neutral evolution. But prior to that, one more thing to take care of...

Evolution lacks foresight; evolution is not engineering
First of all, one must note that a modern function of any given system may not necessarily have been there at the initial stages of evolution. In fact, it is often counterproductive to even assume so. A nice example would be diatom sex.

Upon each division, one of the diatoms gets smaller. The cell is surrounded by two valves: a larger top valve and a smaller bottom one. During division, the bottom one actually becomes the top in the daughter cell. After several generations, some diatom offspring get a little on the small side. Luckily, sex makes them bigger; ie. they produce gametes (or swap nuclei), fuse and make a brand new maximum-sized cell. Jennifer Frazer wrote an awesome post on this topic.

One may look at diatoms and say: What is the function of sex? If you remove sex, the diatoms can't get bigger again, and die a miniscule death. Thus, sex must be there to get bigger!

However, one must imagine evolution as a blind step-by-step process, devoid of any foresight or momentum whatsoever. A common fallacy would be to think of the diatoms first having a problem, and then having to come up with an emergency solution to it, eg. evolve sex. This may seem obviously ridiculous in the case of something as complex as sex, but is often assumed for simpler cases, like evolving a resistance to something. Perhaps we get this picture from the antibiotic resistance examples in bacteria; however, antibiotic resistance is generally much too simple, and bacteria much too numerous, to apply this mode of evolution to everything else. It is additionally pretty rare, but we don't notice the vastly overwhelming multitude of unsuccessfulcases.

Back to our diatoms, the more plausible scenario is actually that sex was there first, and was able to correct for the problems caused by this rather suboptimal mode of mitosis. Sex enabled this peculiar life style; it did not evolve in response to it. 'Enable' is a word that must be used much more frequently in the literature. Certain situations enable certain mutations or other changes to persist or excalate into fixation (either by drift or selection). They do not actually push them there.

Again, evolution cannot anticipate.

Two meanings of 'function'
As a brief aside, it is important to note two distinct meanings of the term 'function', often used rather carelessly:
1. Selected function - what a certain trait would have been selected for in its evolutionary past.
2. Current function - based upon what would happen were the trait removed in the present.

Going back to our diatom example above, the current function of sex in diatoms can be argued as a way to increase the population size back to original levels; for inhibiting sex would remove a way for the organisms to get bigger again. However, this is not the selected function of sex, since it must have already existed before the size problem happened. (the selected function of sex, if any, remains a fuzzy, murky mess)

Positive vs. negative selection
One more brief thing to clean up: 'types' of selection
Negative (aka purifying) selection - selection acting against a trait
Positive selection - selection promoting a trait in a population, usually through competition (the type most commonly spoken of in popular media, despite being far less common to the point of relative rarity...)

Ultimately, positive selection is a form of negative selection where the appearance of a fitter form of a trait renders the rest of the variants relatively less fit, resulting in them being selected against (negative selection). Thus, selection isn't actually ever for anything, strictly speaking. Selection is a constraint, weeding out variants that are insufficiently fit. Furthermore, selection is always lurking about in background, albeit in varying intensities depending on the conditions (see Part I). That said, one must not ever conflate selection with adaptation -- they are not the same thing by any means!

Rise of complexity through non-adaptive means
I won't go into much detail here as I'm sure Arlin Stoltzfus himself will explain it much better in his upcoming posts on Sandwalk. Also, unlike me, he's actually qualified to write about this stuff. I will give a crude overview (to the best of my understanding) along with a few concrete examples. For an additional source on this, I blogged Ford Doolittle's seminar talk on the subject here. The non-adaptive evolution of complexity requires tinkering, relaxed selection (eg. due to smaller effective population size) and ratchets. Tinkering is basic (as mentioned above, evolution lacks foresight, many adaptations are far from optimal as relics of past functions are retained, etc) so I won't discuss it. Small population sizes were discussed in Part I, so now we need the final piece: Ratchets. This is where Constructive Neutral Evolution enters.

In a nutshell, chance interactions may happen to compensate for otherwise-deleterious mutations, thereby enabling them to eventually occur, thereby ultimately resulting in an irreversible dependency upon the interaction. That way, complexity (loosely defined as number of components and interactions within a specified system; as in Lukes et al 2009 PNAS) can increase without ever actually being adaptive. This mechanism stresses that not all complexity is actually 'better', and perhaps much of it may well be a case of mere bloating, much like the bureaucracy of an institution with time. For a system that is required to be constitutively functional, it is in fact easier to bloat complexity than to trim it down, partly just due to basic combinatorics: there are many more ways of being complicated than being simple, and just statistically there'd be more viable states of higher complexity.

Overview of Constructive Neutral Evolution. Modified and enhanced from older diagram here; Ford Doolittle uses something similar in his talk, so it shouldn't be too far off.

This model, while being employed more in molecular biology, is actually applicable universally. Ratchets occur in ecology (someone brought up ecological specialisation as an example), sociology (your favourite institutional bureaucracy), and even evolutionary linguistics (eg. many types of change are irreversable or unlikely to be reversed). Going back to our non-anticipatory step-by-step evolutionary thinking: constructive neutral evolution is powerful. It provides the 'push' where adaptation cannot explain a particular increase in complexity. Ratchets provide an appearance of directionality to a system.

Cyt-18 and the N.crassa mitochondrial self-splicing intron
I will discuss the not-so-self-splicing intron examples in further detail in part III, but just to provide a quite example to the above point, let's look at a Neurospora mitochondrial self-splicing intron that developed a dependency on another protein. This example is based on an old-ish paper, Akins & Lambowitz 1987 Cell. It was found that mutants of cyt-18 exhibited defects in the splicing of group I (self-splicing) introns. Curiously, cyt-18 turned out to be homologous to tRNA synthetases. Further work confirmed that cyt-18 is necessary for splicing in N.crassa, and phylogenies showed it to be a derived trait. That is, in closely related lineages, cyt-18 is NOT necessary for group I intron splicing.

Now the question is, why would N.crassa require an additional protein to perform the same process its relatives can do without involving extra bits. The knee-jerk adaptationist reaction would be to think of it as being somehow better that the simple fully-self-splicing variant. Perhaps the use of a protein enables a better regulation of splicing. For some reason, any peculiar complexity in genetics has to be there for regulation. Apparently, evolution is directionless but still strives for higher complexity of regulatory systems, if you listen to molecular geneticists. However, is this necessarily true for all instances of higher complexity of interactions? How else could complex interactions arise if not for the improvement of a system?

This is where our friendly neighbourhood ratchet, constructive neutral evolution, comes in. Suppose initially the group I intron spliced itself out without the help of any proteins. Just incidentally, a random protein, in this case cyt-18, just happened to bind to it at times. Anyone who's worked with yeast-two-hybrid systems or done immunoprecipitation would be painfully aware of 'false' interactions; that is, when proteins interact biochemically but without any biological significance; or very rarely bind in vivo to begin with. The network of such fortuitous interactions is vast, and increases rapidly as more components are involved -- a positive feedback loop.

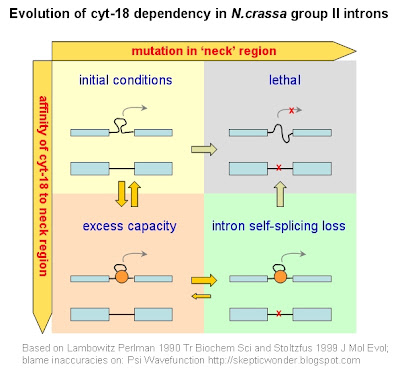
In the Akins & Lambowitz example, the self-splicing intron needs to form a particular secondary RNA structure to remove itself. For the sake of simplicity, let's pretend it has a single neck leading to a loop. The neck needs to form properly in order for the splicing to work, so any mutation destabilising the neck would be lethal. This means these mutations are 'impossible' in the evolutionary sense, as we're unlikely to ever see them.

Now let's say this cyt-18 protein happens to bind to the neck region, and stabilise it slightly. In the grand scheme of things, the intron can splice out properly regardless of whether this protein is there, so it doesn't increase fitness in any way. However, what this protein does to is create an excess capacity in the system by enabling certain otherwise-deleterious mutations to arise in the neck region by compensating their destabilisation effects. Once such a mutation occurs (and it's bound to happen eventually), the lineage now depends upon cyt-18 for proper splicing to occur. Since the chance of the mutation being reverse is quite small, and often even less than the chance of another otherwise-deleterious mutation further fixing the protein dependency, the system is now stuck depending on cyt-18, with no adaptive advantage whatsoever. In a diagram:

N.crassa mitochondrial self-splicing intron example of constructive neutral evolution. See text. Based on Akins & Lambowitz 1987 Cell, Lambowitz & Perlman 1990 Tr Biochem Sci, Stoltzfus 1999 J Mol Evol.

In such a manner, interactions can rapidly accumulate and form the ridiculously intricate pathways that horrify biochemists, geneticists and cell biologists alike, not to mention anyone working with 'transcriptomes' and 'proteomes' and (ewww) 'interactomes'. Not all of these complex pathways are that way for adaptive reasons, despite the common assumption. Some of these complexities can later be exapted for adaptive reasons, sure, but arguably most didn't initially arise adaptively. See Lynch 2007 Nat Rev Genet for a review on neutral evolution of gene interaction pathways.

My hunch at the moment, which may or may not have anything to do with reality, is that most complexity initially may arise through constructive neutral evolution, and some of it later drifts into doing something useful, upon which the lineage fixes a dependency, occasionally through 'positive' selection. Neutral explanations for complexity alleviate the need for awkward scenarios where an organism desperately needs to evolve something quickly as a response. The chance that the right features evolve at the right time, and not before the whole lineage dies off, is usually not very high. But when a lineage has been 'preadapted' through such neutral means, it wouldn't be as adversely affected by changes, or by finding a new niche, or whatever. Evolutionary adaptation is not a particularly efficient response mechanism, but neutral evolution is a wonderful source of 'enabling' modifications (excess capacities) that can later be molded into apparently functional parts. The explosion of complexity is controlled by negative selection, preventing it from getting too extreme and costly, although in organisms with smaller effective population sizes (where drift often overpowers selection; see Part I), complexity can get quite extreme nonetheless.

Most supporters of neutral theories and pluralism perhaps wouldn't be as extreme though, so don't take the above paragraph too seriously. In Part III, I will discuss further examples, including the little that is known about the evolution of ciliate nuclear dimorphism as well as gene scrambling, which was the original topic that sparked this discussion. Furthermore, I'd like to try and extrapolate this model beyond molecular biology, venturing a bit into evolutionary linguistics, which may also be teeming with ratchets. Hopefully by now you'd see that the concept of neutral evolution being capable of driving complexity is at the very least worth considering.

As Michael Lynch pointed out (eg. 2007 PNAS), selection may very well not be the sole source of order and complexity. In some cases, perhaps not even the dominant one.

References
Akins, R., & Lambowitz, A. (1987). A protein required for splicing group I introns in Neurospora mitochondria is mitochondrial tyrosyl-tRNA synthetase or a derivative thereof Cell, 50 (3), 331-345 DOI: 10.1016/0092-8674(87)90488-0

LAMBOWITZ, A., & PERLMAN, P. (1990). Involvement of aminoacyl-tRNA synthetases and other proteins in group I and group II intron splicing Trends in Biochemical Sciences, 15 (11), 440-444 DOI: 10.1016/0968-0004(90)90283-H

Lukes J, Leander BS, & Keeling PJ (2009). Cascades of convergent evolution: the corresponding evolutionary histories of euglenozoans and dinoflagellates. Proceedings of the National Academy of Sciences of the United States of America, 106 Suppl 1, 9963-70 PMID: 19528647

Lynch, M. (2007). Colloquium Papers: The frailty of adaptive hypotheses for the origins of organismal complexity Proceedings of the National Academy of Sciences, 104 (suppl_1), 8597-8604 DOI: 10.1073/pnas.0702207104

Lynch, M. (2007). The evolution of genetic networks by non-adaptive processes Nature Reviews Genetics, 8 (10), 803-813 DOI: 10.1038/nrg2192

Pinker S, & Bloom P (1990). Natural language and natural selection Behavioral and brain sciences, 13 (4), 707-784

Stoltzfus, A. (1999). On the Possibility of Constructive Neutral Evolution Journal of Molecular Evolution, 49 (2), 169-181 DOI: 10.1007/PL00006540

Sunday Protist -- Notodendrodes: giant tree forams

Foraminifera are wonderful organisms. For a glimpse of their phylogeny, see this diagram, but keep in mind that the majority of forams are actually allogromiids, forams which build their walls of protein as opposed to scavenged material or depositing mineral substances. From the allogromiids there have been several independent origins of non-proteinaceous forams, many building their tests out of sand grains, remnants of prey or their own waste. Test-building is a complicated and highly regulated process (many forams actually select sand grains with the right properties for building their tests!), a topic I should get around to eventually (not with those dark menacing storm clouds rapidly approaching from the horizon signalling the inevitable Armageddon finals). Thus, I figured that for this superficial protist appreciation post one can't go wrong with Notodendrodes, a genus of forams that look like trees!

Notodendrodes, like their sphaerical relative Rhabdammina, build their tests out of sand grains, especially quartz. Unlike Rhabdammina, they also have extensive "root" and "arborescent" structures sticking out of the sphaerical shell and into the sand and up in the air, respectively.

Notodendrodes antarctikos from the deep sea, arborescent structure. Image from Bowser lab, shamelessly stolen from certain course slides.

One must also note that forams extend far beyond their tests: they are surrounded by a complex network of extruded strands of cytoplasm forming the reticulopodia. These networks can be used to capture prey, absorb nutrients and, in some species, transport algal symbionts far outside the shell to harvest light energy. Notodendrodes lives too deep for housing photosynthetic symbionts; it is said to use its root pseudopodia for absorbing nutrients from the sediment and the arborescent network for sifting through the algal rain falling from the surface (Bowser Lab webpage on Notodendrodes ).

Notodendrodes hyalinosphaira. Scalebars: A,B - 2mm; C - 1cm; D - 5mm (DeLaca et al. 2002 J Foram Res)

These cells are quite sophisticated and should make great companions for cell biology research. The reticulopodia are able to move things along them (seems to be widespread feature among Rhizarians), and before you get the idea that these giant cells are docile and harmless, some forams can prey on small animals like copepods. There are some truly frightening micrographs in OR Anderson's Biology of Foraminifera.

Notodendrodes is apparently uninucleate. Wonder what ploidy levels would be needed to sustain such a monster-sized cell...

Anyway, this post fails to do justice to these organisms, but this week is simply awful for me, so I must leave it at that. My whole life is due this week. Also, I have three weeks left to finish wrapping up my current research project, and I'm having great difficulty focusing on it with all the course-related crap on top of it. Expect negligible blogging efforts in the next few weeks...

By the way, Mystery Micrograph #20 feels neglected. Do you guys need a few more micrographs for help?

Meanwhile, some random foram stuff to look at:

References
Bowser, S. (1995). Larger agglutinated foraminifera of McMurdo Sound, Antarctica: Are Astrammina rara and Notodendrodes antarctikos allogromiids incognito? Marine Micropaleontology, 26 (1-4), 75-88 DOI: 10.1016/0377-8398(95)00024-0

DeLaca, T. et al. (2002). NOTODENDRODES HYALINOSPHAIRA (SP. NOV.): STRUCTURE AND AUTECOLOGY OF AN ALLOGROMIID-LIKE AGGLUTINATED FORAMINIFER The Journal of Foraminiferal Research, 32 (2), 177-187 DOI: 10.2113/0320177

Irremediable Complexity: Notes from Ford Doolittle's seminar talk

While I work on polishing up Part II of the Neutral Evolution series, thought I'd write up and post my four pages of notes from Ford Doolittle's seminar talk today yesterday, while I can still remember what my scribbles were supposed to mean. As there's no unpublished data there, and a long-awaited paper on the subject has just been submitted, I believe it should be fair game for blogging. Coming from a vicious field (Arabidopsis, sigh...), I'm generally rather cautious about blogging department talks and such, but Constructive Neutral Evolution is a subject in need to spreading, and not a particularly competitive area at the moment...

Rosie has another summary of today's yesterday's talk, with an executive summary therein; she tried to scoop me, so clearly this means I must outdo her in length and verbosity =P

[If anything doesn't make sense, it's very likely an error on my part]
-----
Irremediable Complexity - Ford Doolittle, 07 Apr 2010
[paraphrased from notes; own comments in grey]
- Is each step in the evolution of a complex machine useful?

Irremediable complexity involves three factors: Tinkering, small populations, ratchets (Constructive Neutral Evolution). [prior to that, must discuss common views on complexity first]

Common views on complexity
- Directionality: 19th century - divine forces guide evolution; 20th century - orthogenesis - evolution exhibits a drive towards perfection (and complexity)
- Progress: Life started off being simple and became increasingly complex
But is there necessarily a trend?
(Gould 1996 Full House) The Drunkard's Walk: if one starts off at a limit that cannot be passed, random steps will eventually lead away from this limit. Presumably, life began more or less at the lower limit of complexity (specialised parasites aside), so it's bound to get more complex as it's the only way to go.
In fact, complexity is increased only in a few lineages, which also happen to be the ones we really like to look at.

So is the evolution of multicellular animals and plants from choanoflagellate-like and chlamydomonas-like organisms, respectively, a drunkard's walk or driven by something (eg. selection)?

Selectionist explanations
- Accumulation of specific adaptations results in complexity (eg. The Eye)
Another example: larger genome size is an adaptation for more gene regulation which is required in more complex organisms. [Note: C-value paradox, etc] Molecular biologists have an obsession with 'mystery DNA' having regulatory roles...
- Arms races, sexual selection
Greater biodiversity/more competition between organisms stimulates greater complexity, eg through niche specialisation and sex selection
- Evolving evolvability
Outdoing one's environmental changes by evolving faster. Eg. Exon shuffling as a function of introns: introns space out exons allowing more novel combinations of these exons to occur, which may be adaptive.
Caveat with evolvability -- it's a clade-selection level trait, not individual level.

Neutral forces - should be our null hypotheses
- Tinkering (François Jacob) -- will still have traces of an apparatus' past functions along with new ones --> life is full of Rube Goldberg machines.
- Small population size -- mildly deleterious traits more likely to be fixed in smaller populations (Michael Lynch; more info in Part I of my Neutral Evolution series) Eukaryotes are a case of smaller population size relative to prokaryotes.
- Ratchets -- 1. Maynard-Smith & Szathmary's Major Transitions; 2. Stoltzfus & Covello's Constructive Neutral Evolution
Major Transitions: There are steps in evolution that are difficult or impossible to reverse -- act as ratchets.

Constructive Neutral Evolution: a previously fortuitous (non-functional) interaction can enable an otherwise-deleterious mutation to occur, resulting in a dependency upon this interaction. [a diagram is in the making]
More interactions evoke more opportunity for Constructive Neutral Evolution to drive (via ratchetting) an increase in complexity. [thus, the result would be an explosion of complexity past a certain threshold]
The dependency can be built up by other mutations, thus further solidifying the requirement for a given interaction.
Note that no positive selection is required at any step [only purifying], would also be more drastic in smaller populations where more deleterious mutations are fixed by drift. That said, positive selection can still play a role in parallel.

Examples:
Lambowitz's maturase-requiring group I self-splicing intron. [will be discussed in further detail in impending post] A derived Neurospora lineage requires a maturase for the splicing of group I introns whereas nearby relatives do not. Lambowitz later (2006) argues that maturase-mediated splicing evolved in response to the splicing problem, as opposed to enabling it to arise. This is putting the cart before the horse.

kDNA editosome (Trypanosomes et al.)
[Can be summed up in one interjection: whyyyyyyyyyyyyy???]
In summary, genes coded by the mitochondrial genome are non-sensical, and right after transcription the pre-mRNAs are edited by the complicated process involving templates and inserting various U's where they are needed.

There are several explanations that have been proposed:
- relic of the RNA world -- for starters, tryps are derived.
- to correct pre-existing mutations -- backwards logic again (cart before the horse)
- regulation
[Digression to discuss the two oft-conflated meanings of function]
1. Selected function -- how a trait got to be there
2. Current function -- what happens if trait is removed

Example from Maynard-Smith: Stiff back of the horse. Removal thereof would prevent humans from riding it, but no one can argue that the horse's back evolved so that humans could ride it in the future!

How editing really arose -- CNE [see Stoltzfus 1999 JME and Lukes et al 2009 PNAS(and subsequent correspondence)]: once the process started, it couldn't be reversed, thus complexity reached an absurd level.
"Absurdly complex spliceosome"
- if you think about it, it's "incredibly stupid" to have such a complex machine for removing introns
- cites "Five Easy Pieces" Sharp 1991 Science laying out a hypothesis for the evolution of group II introns
- see Lambowitz example for how the spliceosome may have arisen through initially-neutral protein interactions

Ribosome
Also by CNE. Roughly put, the RNA does most of the enzymatic work in the ribosome, with the proteins taking on more of a structural function. Presumably, initially the ribosome could've been entirely a ribozyme, picking up various proteins for supporting structural roles, like the Lambowitz intron, with the help of constructive neutral evolution.

Cited TW O'Brien 2003 IUBMB Life paper: the mammalian mitochondrial ribosome is smaller than that of its host (eukaryotic) yet larger than the prokaryotic counterpart; furthermore, many of the extra mitochondrial ribosomal proteins do not come from the eukaryote! This is a great example of convergence between the two separate evolutionary paths, both starting off with the small (at least in terms of protein count) prokaryotic ribosome and becoming bloated in complexity. Furthermore, mitochondria also have a greatly reduced effective population size, thereby encouraging the accumulation of complexity, unlike in their free-living bacterial brethren. [would be interesting to compare plastid, mitochondrial and eukaryotic ribosomal evolution, controlling for LGT, replacement, loss, and all the other crap associated with endosymbiosis, of course. A nice system with at least two independent replicates originating from very distantly-related sources]

[Another guy (unsure about citing personal communications without their knowledge) rather eloquently put it along the lines of "The rRNA was fully functional enzymatically on its own until the other shit stuck along for the ride"]


In closing, tinkering leads to klunkiness, smaller populations allow more mildly deleterious mutations, and ratchets make complexity ultimately unavoidable.

For another example of irremediable complexity, think what would happen if an institution was formed with a few small committees with specific functions and left alone for a few decades. Like a university. The bureaucracy and administrative complexity would increase while the overall efficiency of the system wouldn't benefit much. One can think of the complex biochemical pathways as "cellular bureaucracy".

"Complexity is unavoidable and largely irremediable: Resistance is useless"


-----
My initial impression of Ford Doolittle came from the whole 'missing Tree of Life' debacle, where he did appear rather rash and extremist, perhaps largely due to the media portrayal and associated uproar -- after his seminar talk and a more informal chat at lunch, I fully retract my first impressions, and must say that he's actually quite reasonable and not radical or extremist at all (and very pleasant and interesting to talk to). Naturally, science reporters reporters in general tend to hyperpolarise any slightest argument they chance upon, and turn anyone with a shred of an opinion into a flaming radical; thus it was another lesson to be extremely cautious about impressions you get about someone based on someone else's reporting. But another thing I've noticed is he seems less assertive in person than in his own papers as well. Well-balanced and subtle ideas seldom get the attention they deserve, so they must often be blown out of proportion to be at all noticed.

Perhaps this is another reason neutral theories remain so obscure: the adaptationists are occupied with explaining natural selection to creationists et al., thereby being much noisier and noticeable. The more balanced pluralists don't have much extremist thought to push, so they tend to get ignored (I find the Stoltzfus 1999 paper to be quite subtle and unassertive; perhaps that's why it was largely ignored).

Back to the ToL kerfuffle: If one were to say "LGT is very frequent in bacterial populations and may pose very substantial problems to reconstructing bacterial phylogeny and the deep history of life, perhaps even posing a valid question of whether such a phylogeny may truly ever be found", the statement is too reserved and subtle to make much of a splash beyond a small circle of specialists. However, if one goes all out and shouts "The Tree of Life is dead!", people actually turn around and look. Many misinterpret the message and get their own strange notions on the subject (often believed much more strongly than by the originator of the idea...), but at least some people get it and consider the problem.

Furthermore, the "Darwin was wrong" slant was intended to signal that we should get away from our Darwin fetish. I fully agree. Darwin was a great scientist, but it is outright immoral to ignore the hard work of thousands of people who came after him, and the thousands who are working in the field right now. Darwin may have sparked the field, but he is certainly not its most important element. The term "Darwinism" is vacuous and misleading, and should be abandoned soon. Furthermore, who cares what creationists think? Some of us are sick of having to change our vocabulary just because some religious idiot with an agenda could abuse it. The primary role of evolutionary biologists is to study evolutionary biology; educating the public is secondary (while still important); dealing with creationists is about last. Science educators are responsible for that. We cannot fight religion, especially its fundamentalist forms, with reason (hence why Dawkins fails at it). So what if they misunderstand and misrepresent Darwin? People misunderstand and misrepresent quantum mechanics even more, and yet physicists don't seem to lose sleep over it.

Political agendas will always be there; textbooks will always be influenced by the political (and sadly, religious) climate of the times. It sucks, but such is reality. History and the social sciences are also badly mangled in schools (eg. communism is still a topic not only taught entirely wrong, but also characterised by a blunt refusal to listen to those who may know better). After all, to understand science effectively, one must appreciate the subject, and be willing to not only accept, but commit work to it. The unwilling will never learn unless they want to. What is of a much higher importance than defending Darwin is promoting the overall public image of science and academia in general, and making academic activity 'cool' in the eyes of the public. If scientists were well-respected in 1970's Russia, there's no reason we can't acheive that again and in a different society. But it will take work.

But to get that to work, we must strive to suppress our polarising tendencies and recognise that often people's opinions are more subtle than they appear. We must also pay greater attention to ideas that are not pushed as aggressively as others, such as constructive neutral evolution. Those may well be more refined and ready for acceptance than the ideas cast in apparent simplicity and loudness.

References:
O'Brien, T. (2003). Properties of Human Mitochondrial Ribosomes IUBMB Life (International Union of Biochemistry and Molecular Biology: Life), 55 (9), 505-513 DOI: 10.1080/15216540310001626610

Sharp PA (1991). "Five easy pieces". Science (New York, N.Y.), 254 (5032) PMID: 1948046

Stoltzfus, A. (1999). On the Possibility of Constructive Neutral Evolution Journal of Molecular Evolution, 49 (2), 169-181 DOI: 10.1007/PL00006540

Slow blogging alert...

As you may or may not have noticed, it's April. April is a very special time for some poor fucks students. This is where this wonderful bi-/tri-annual hazing ritual occurs wherein a tribesman is placed before a patterned sheet of paper and scribbles along for a predetermined duration of time, Subsequently, a tribesman of a higher rank employs these scribbled sheets of paper in a peculiar ritual of divination rite, wherein markings (usually in red ink) are splattered all over to determine the worth (and fate) of the tribesman in question. A certain number of these rituals must be committed over 4-6 years before the tribesman has accomplished the initation rite successfully, upon which he or she dons peculiar medieval robes and is said to now be of a higher rank. These robes seem to reflect the colouration scheme of the respective clan the tribesman belongs to.

Long story short, I haz finals looming ahead. April isn't as bad as December (we actually get to see sunlight, which is kind of cool), but I must also wrap up my current project and write everything up, and as you may know, wrapping up one's research can be an epic pain in the ass. Why does it seem easier to write up other people's research rather than your own?

Also, there's like term papers and presentations and stuff. And taxes. And other gov't paperwork. And holy crap I don't wanna think about how I'm gonna survive this month. Thus, blogging will probably be reduced, and happen [even more] in sporadic bursts (procrastination is sort of quantised...). Kind of stressed at the moment, and the more stuff I have to do, the less I can focus on any given item in the list. Really annoying, to be honest.

That said, Sunday Protist and the continuation to the Neutral Evolution posts are on their way, and apologies for the delay. Actually, I think I'll wait until Wed to finish the next installment on Constructive Neutral Evolution, as Ford Doolittle is giving a talk on that at a dept seminar (sooo excited!) Would make sense to blog about that after his talk.

But yeah, apologies in advance for sub-par blogging until May. And why do I have to absorb the Canadian obsession with incessant apologising despite not actually being Canadian? Grrr...sorry about that! =P